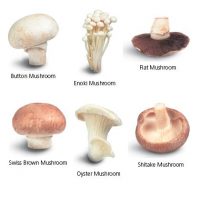
Edible and medicinal mushrooms (macrofungi belonging primarily to the phyla Basidiomycota and Ascomycota) occupy a taxonomically unique biological kingdom that bridges the nutritional characteristics of plants and animals. Rather than synthesizing cellulose or storage starches, fungi construct their cellular architecture from structural chitin and branched beta-glucans, yielding a low-caloric, fat-free, and cholesterol-free functional food matrix delivering exceptional micronutrient density. Grounded in modern fungal biochemistry and human clinical trials, whole culinary and medicinal mushrooms provide 6 primary evidence-based health benefits: orchestrating innate and adaptive immune surveillance via beta-(1,3/1,6)-D-glucan binding to myeloid Dectin-1 and complement receptor 3 (CR3), conferring profound mitochondrial cytoprotection through the dietary antioxidant L-ergothioneine utilizing the dedicated human transporter SLC22A4 (OCTN1), supplying UV-bioavailable ergocalciferol (vitamin D2) to sustain circulating 25-hydroxyvitamin D concentrations, attenuating serum atherogenic lipoproteins through intestinal bile acid sequestration and endogenous fungal statins, feeding prebiotic mycopolysaccharides to commensal gut microbiota to drive short-chain fatty acid (SCFA) synthesis, and optimizing postprandial satiety signaling and metabolic weight regulation through high-volume, low-energy-density protein displacement.
Quick Nutrition Science & Key Takeaways
- Targeted Immune Receptor Surveillance: Fungal cell-wall beta-(1,3/1,6)-glucans act as biological pathogen-associated molecular patterns (PAMPs), binding directly to Dectin-1 receptors on macrophages and dendritic cells to prime natural killer (NK) cell cytotoxicity without inducing systemic hyper-inflammation.
- Dedicated Human Ergothioneine Transport: Mushrooms represent the primary dietary source of L-ergothioneine, a unique thiol-histidine antioxidant that is actively concentrated into mitochondria via the human OCTN1/SLC22A4 transporter to neutralize hydroxyl radicals and protect vascular endothelial DNA.
- Photobiological Vitamin D2 Biosynthesis: Fungi contain high concentrations of the membrane sterol ergosterol, which converts into bioavailable vitamin D2 (ergocalciferol) upon brief exposure to ultraviolet light (UVB), rivaling supplemental cholecalciferol in raising serum 25(OH)D levels.
- Cardiometabolic & Glycemic Resilience: Soluble mycopolysaccharides, chitinous fibers, and naturally occurring lovastatin (in species such as Pleurotus ostreatus) lower circulating apolipoprotein B and suppress postprandial glycemic excursions.

Fungal Biochemistry: The Chitinous Matrix, Beta-Glucans, and Ergothioneine
Unlike vascular plants whose cell walls are composed of cellulose, pectin, and lignin, fungal cell walls are structured around a rigid, three-dimensional fibrillar network of chitin (poly-β-(1→4)-N-acetyl-D-glucosamine) cross-linked to highly branched β-(1→3)- and β-(1→6)-D-glucans, mannans, and glycoproteins. This specialized skeletal matrix makes raw mushrooms tough and resistant to human gastrointestinal enzymes, necessitating thermal processing (cooking) to disrupt chitinous fibrils and liberate the intracellular bioactive nutrients.
From a molecular perspective, mushrooms produce two classes of compounds that are virtually absent in standard plant foods. The first is L-ergothioneine (ESH), a sulfur-containing amino acid derivative synthesized almost exclusively by fungi and certain actinobacteria. The human body expresses an evolutionarily conserved, highly specific organic cation transporter, OCTN1 (encoded by the SLC22A4 gene), whose primary physiological substrate is ergothioneine. OCTN1 actively transports ESH across plasma membranes and concentrates it within vulnerable cellular compartments—specifically the inner mitochondrial membrane and erythrocyte cytosol—where it quenches hydroxyl radicals (OH•), singlet oxygen (1O2), and hypochlorous acid (HOCl) far more effectively than glutathione or alpha-tocopherol.
The second distinctive fungal feature is the presence of ergosterol (provitamin D2) embedded within fungal plasma membranes. When exposed to ultraviolet radiation (specifically UVB photons in the 280–315 nm spectrum), ergosterol undergoes photolytic electrocyclic ring-opening to yield previtamin D2, which spontaneously isomerizes at room temperature into ergocalciferol (vitamin D2). Peer-reviewed mycological trials indexed by the National Institutes of Health (NIH) on mushrooms as a dietary source of vitamin D indicate that 100 grams of UVB-exposed white button or shiitake mushrooms can deliver between 400 IU and 1,000 IU of biologically active vitamin D2, offering an effective vegetarian alternative to fish oils and cholecalciferol.
“Mushrooms represent a distinct biochemical kingdom whose fungal beta-glucans and mitochondrial ergothioneine operate through specialized human receptors and transporters that plants cannot activate.”
6 Science-Backed Health Benefits of Culinary & Medicinal Mushrooms
Contemporary clinical investigations and nutritional biochemistry confirm 6 distinct, evidence-backed physiological benefits provided by regular mushroom consumption:
1. Beta-Glucan Immunomodulation & Dectin-1 Receptor Surveillance
The primary mechanism underlying mushroom-mediated immune defense centers upon high-molecular-weight beta-(1,3/1,6)-D-glucans. When ingested, these non-digestible polysaccharides transit through the upper digestive tract and are sampled by intestinal M-cells within the Peyer’s patches of the ileum. Myeloid dendritic cells and resident macrophages internalize and fragment the beta-glucans, presenting the oligosaccharide motifs to cell-surface pattern recognition receptors (PRRs), predominantly Dectin-1 (CLEC7A) and Complement Receptor 3 (CR3 / CD11b/CD18).
As documented in immunology research published by the National Center for Biotechnology Information (NCBI) on beta-glucan immunomodulatory activities, Dectin-1 ligation initiates an intracellular signaling cascade via immunoreceptor tyrosine-based activation-like motifs (ITAMs) and spleen tyrosine kinase (Syk). This primes circulating natural killer (NK) cells, increases the phagocytic index of polymorphonuclear neutrophils, and upregulates baseline antiviral cytokine production (interferon-gamma, IL-12) without triggering dysregulated inflammatory storms. Regular consumption of cultivated culinary species (such as Agaricus bisporus, Lentinula edodes, and Pleurotus ostreatus) directly supports human host defense during acute respiratory pathogen challenges.
2. Cellular Ergothioneine & Mitochondrial Antioxidant Defense
Oxidative phosphorylation within human mitochondria inevitably leaks single electrons to molecular oxygen, generating superoxide anions (O2•−) that compromise mitochondrial DNA, oxidize respiratory complexes I and III, and accelerate cellular senescence. While classical antioxidants like vitamin C are rapidly metabolized, L-ergothioneine exhibits exceptional intracellular stability and does not auto-oxidize into pro-oxidant intermediates.
Because human cells express the dedicated OCTN1 / SLC22A4 transporter, dietary ergothioneine from mushrooms is avidly absorbed in the proximal small intestine and concentrated within tissues subject to high oxidative fluxes, including hepatocytes, renal proximal tubular cells, central neurons, and vascular endothelial cells. Epidemiological and laboratory studies demonstrate that higher tissue ergothioneine concentrations correlate with lower levels of systemic lipid peroxidation, decreased F2-isoprostanes, and preservation of microvascular endothelial nitric oxide synthase (eNOS) activity. Learn more about foundational cellular defense in our detailed guide on antioxidant phenolics and cellular protection.
3. Ergosterol Photobiology & Bioavailable Vitamin D2 Synthesis
Vitamin D deficiency remains a widespread public health crisis, impacting skeletal mineralization, immune function, and endocrine homeostasis. Because plants do not synthesize vitamin D, dietary sources are historically restricted to animal tissues (fatty fish, egg yolks) and fortified dairy products. Mushrooms are the only non-animal whole food capable of generating physiologically meaningful quantities of vitamin D.
Upon exposure to natural sunlight or industrial UVB irradiation, fungal ergosterol transforms into previtamin D2 and subsequently ergocalciferol (vitamin D2). Once absorbed via mixed lipid micelles in the intestinal lumen, vitamin D2 binds to vitamin D-binding protein (DBP), enters hepatic circulation, and undergoes sequential 25-hydroxylation by CYP2R1 and 1α-hydroxylation by renal CYP27B1 to form the active hormone 1,25-dihydroxyvitamin D2 [1,25(OH)2D2]. Clinical crossover trials demonstrate that consuming 100 grams of UVB-pulsed white button mushrooms daily is just as effective as an oral 2,000 IU vitamin D2 supplement in sustaining wintertime circulating 25(OH)D levels. For comprehensive management of systemic skeletal risks, explore our protocol on vitamin D deficiency symptoms and clinical management.
4. Cardiometabolic Support & Bile Acid Sequestration
Mushrooms exert potent cardioprotective effects through a dual biochemical pathway involving physical intestinal clearance and endogenous lipid enzyme inhibition. First, the soluble fraction of fungal beta-glucans and insoluble chitin fibrils form a viscous unstirred water layer along the duodenal epithelium, entrapping conjugated bile acid micelles and promoting their fecal excretion. To replenish the bile acid pool, hepatocytes must upregulate cholesterol 7α-hydroxylase (CYP7A1), drawing cholesterol from circulating low-density lipoprotein (LDL) particles via upregulated hepatic LDL receptors.
Second, specific edible fungi—most notably oyster mushrooms (Pleurotus ostreatus)—naturally synthesize small, physiological quantities of lovastatin (monacolin K). This fungal polyketide acts as a competitive inhibitor of 3-hydroxy-3-methylglutaryl-coenzyme A (HMG-CoA) reductase, the rate-limiting enzyme in hepatic cholesterol biosynthesis. Combined with high concentrations of potassium (~300–450 mg per 100 g) and near-zero sodium, mushrooms help lower arterial peripheral resistance, supporting normal blood pressure regulation and endothelial flexibility.
5. Prebiotic Polysaccharides & Gut Microbiota Homeostasis
Because the human genome lacks the necessary glycolytic enzymes (chitinases and beta-glucanases) to break down the dense fungal cell walls, the majority of mushroom carbohydrates reach the distal cecum and colon intact. There, they function as non-digestible prebiotic substrates for the colonic microbiome.
Beneficial commensal taxa—particularly Bifidobacterium, Faecalibacterium prausnitzii, and Roseburia—ferment mushroom polysaccharides into short-chain fatty acids (SCFAs), predominantly acetate, propionate, and butyrate. Butyrate serves as the primary metabolic fuel for colonic colonocytes, reinforcing claudin and occludin tight-junction protein assembly to prevent gut hyper-permeability (endotoxemia). Concurrently, propionate transits to the liver via the portal vein, where it inhibits fatty acid synthesis and enhances systemic insulin sensitivity. For insights on optimizing dietary fiber and metabolic satiety, review our evidence-based overview on protein kinetics and nutrient-dense whole-food matrices.
6. Satiety Kinetics & Caloric Density in Metabolic Weight Management
Obesity and metabolic syndrome are heavily driven by the hyper-palatable, energy-dense Western dietary matrix. Edible mushrooms possess an exceptionally low caloric density (approximately 22 to 28 kcal per 100 grams) accompanied by high moisture content (~90%), structural fiber, and umami-rich ribonucleotides (guanosine 5’-monophosphate) and free glutamic acid.
In randomized controlled feeding trials, substituting standard 80/20 ground beef with chopped white button or portobello mushrooms (a culinary strategy known as the “blend and substitute” paradigm) resulted in an involuntary daily reduction of 400 to 500 calories without compromising subjective meal volume, chewiness, or palatability. The mechanical volume of the fungal meal stimulates gastric stretch mechanoreceptors (vagal afferent signals), promoting early postprandial secretion of the satiety peptides cholecystokinin (CCK) and peptide YY (PYY) while depressing the hunger hormone ghrelin. Explore the science of caloric deficit dynamics in our analysis of weight loss myths and metabolic adaptation.
Comparative Matrix: Fungal Bioactives, Molecular Targets & Physiological Impact
The following multi-dimensional comparative matrix outlines the primary bioactive components across common culinary and medicinal mushroom varieties, their precise physiological targets, underlying biochemical mechanisms, and clinical evidence ratings:
| Mushroom Variety / Bioactive | Primary Physiological Target | Biochemical Mechanism & Molecular Action | Evidence Level & Dietary Guidance |
|---|---|---|---|
| 1. White Button & Cremini (Agaricus bisporus) | Intestinal M-Cells & Dectin-1 Receptors | Supplies beta-(1,3/1,6)-glucans that bind Dectin-1 on macrophages, priming innate NK cell activity and mucosal sIgA. | Level I: Readily available everyday staple; light sautéing optimizes glucan bioaccessibility. |
| 2. L-Ergothioneine (Porcini, Shiitake, Oyster) | Mitochondrial Matrix via SLC22A4 (OCTN1) | Actively concentrates in mitochondrial membranes, neutralizing hydroxyl radicals (OH•) and protecting mtDNA. | Level I/II: Outstanding cellular longevity antioxidant; resistant to standard culinary heat. |
| 3. UVB-Pulsed Mushrooms (Ergocalciferol) | Duodenal TRPV6 Channels & Hepatic CYP2R1 | Photolytic conversion of ergosterol to vitamin D2; 25-hydroxylation elevates circulating serum 25(OH)D. | Level I: 100 g of sun-exposed mushrooms delivers 400–1,000 IU bioavailable vitamin D. |
| 4. Oyster Mushrooms (Pleurotus ostreatus) | Hepatic HMG-CoA Reductase & Bile Acid Pool | Naturally contains trace lovastatin and viscous beta-glucans, inhibiting endogenous sterol synthesis and increasing fecal bile loss. | Level II: Demonstrably reduces total and LDL cholesterol in hyperlipidemic cohorts. |
| 5. Shiitake Lentinan & Prebiotic Fibers | Colonic Microbiota & Colonocyte Tight Junctions | Selectively fermented by Bifidobacterium into butyrate and propionate, suppressing intestinal endotoxemia. | Level II: Supports microbiome diversity, mucosal integrity, and systemic glycemic stability. |
| 6. Portobello Whole-Food Meat Substitute | Gastric Vagal Mechanoreceptors & Enteroendocrine L-Cells | Displaces high-fat animal proteins; activates PYY and CCK release while lowering daily energy intake by 400+ kcal. | Level I: Clinically proven culinary strategy for long-term sustainable fat loss and metabolic regulation. |
Debunking Raw Mushrooms, Wild Foraging, and Cancer “Miracle Cure” Myths
Modern clinical evidence and toxicology urge discernment regarding pervasive cultural myths surrounding mushrooms:
- Myth 1: Raw mushrooms in salads are healthier than cooked mushrooms. Raw mushrooms contain agaritine, a heat-labile phenylhydrazine derivative found in Agaricus bisporus that exhibits potential mutational toxicity in animal assays. Furthermore, raw fungal cell walls are bound by indigestible chitin, locking away beta-glucans and micronutrients. Sautéing, steaming, or simmering mushrooms for 5 to 10 minutes degrades over 90% of agaritine, softens chitin fibrils, and dramatically increases the bioavailability of both beta-glucans and ergothioneine.
- Myth 2: Any wild mushroom that smells pleasant is safe to forage. This dangerous assumption accounts for hundreds of severe poisonings annually. Highly lethal species such as Amanita phalloides (the Death Cap) contain amatoxins (α-amanitin), which are entirely heat-stable, odorless, and pleasant-tasting. As little as half a mushroom cap contains enough amatoxin to irreversibly halt RNA polymerase II transcription in human hepatocytes, culminating in fulminant hepatic necrosis, acute kidney failure, and death. Never forage wild mushrooms without formal mycological credentials.
- Myth 3: Medicinal mushroom extracts can replace conventional oncology treatments. While purified beta-glucans (such as Lentinan and Krestin/PSK) are approved in Japan and other jurisdictions as adjunctive immunotherapies administered alongside conventional chemotherapy to mitigate leukopenia and support immune surveillance, raw mushroom powders or commercial tinctures do not “cure” solid tumors. Claiming that oral supplements can substitute for oncology care is dangerous and medically unfounded.
Disclaimer: This article is for informational purposes only and is not intended as medical advice. Always consult with a qualified healthcare professional before making changes to your health regimen.
Frequently Asked Questions (FAQ)
Can mushrooms provide enough vitamin D for individuals with limited sun exposure?
Yes, provided the mushrooms have been exposed to ultraviolet light. Naturally cultivated indoor mushrooms contain minimal vitamin D; however, placing sliced white button, cremini, or portobello mushrooms gills-up in direct mid-day sunlight for 15 to 30 minutes (or purchasing commercially UVB-treated mushrooms) converts cellular ergosterol into 400 to 1,000 IU of bioavailable vitamin D2 per 100 grams, meeting 100% of the recommended daily intake.
Why should mushrooms always be thoroughly cooked before consumption?
Cooking is essential for two key biological reasons: degradation of natural toxins and nutrient bioavailability. Raw button mushrooms contain small quantities of agaritine, a natural hydrazine compound that is readily deactivated by heat. Furthermore, fungal nutrients are encased in tough chitinous cell walls that human enzymes cannot break down; gentle heat softens these walls, liberating beta-glucans, antioxidants, and minerals for intestinal absorption.
How do mushroom beta-glucans differ from grain beta-glucans like oats?
Mushroom and oat beta-glucans feature distinct structural linkages that dictate their physiological actions. Oat beta-glucans possess linear β-(1→3) and β-(1→4) linkages, primarily functioning mechanically in the gut to bind bile acids and slow carbohydrate uptake. In contrast, fungal beta-glucans possess complex β-(1→3) backbones with β-(1→6) branch points, a molecular conformation that specifically matches human Dectin-1 and CR3 pattern recognition receptors to stimulate immune cell signaling.
Are medicinal mushroom powders and extracts safe for everyone to take?
While culinary mushrooms are safe for virtually all adults, concentrated medicinal extracts (such as Reishi, Chaga, or Cordyceps) possess potent pharmacodynamic properties. They can inhibit platelet aggregation, potentiating the effects of blood-thinning medications (warfarin, aspirin), and can stimulate lymphocyte proliferation, posing risks for individuals with systemic autoimmune conditions or those on immunosuppressant therapies. Always consult your physician before initiating concentrated mycological supplements.